
Kiwifruit bud physiology and flower differentiation

Savvas Pastopoulos, Agronomist MSc, Pastopoulos Agronomics, Neos Mylotopos, Pella, Greece
A kiwifruit vine does not decide its flowering in winter. It decides it in June and July of the previous year, inside a bud that shows nothing at the time. Everything that follows, chilling, pruning, fertilisation, does not create flowering; it merely allows or prevents the expression of a decision already taken. That changes how canes are chosen at winter pruning.
- Where exactly kiwifruit bears its crop
- The two-year cycle of the bud
- What is inside a first-order axillary bud
- When flowering is decided: the moment of evocation
- The genetic confirmation
- Dormancy and its three faces
- Chilling hours or chilling units: a costly confusion
- How many buds break, and why
- Breaking dormancy: what the research shows and what is permitted
- Nitrogen, vigour and flowering
- What all this means at pruning
- Sources
1. Where exactly kiwifruit bears its crop
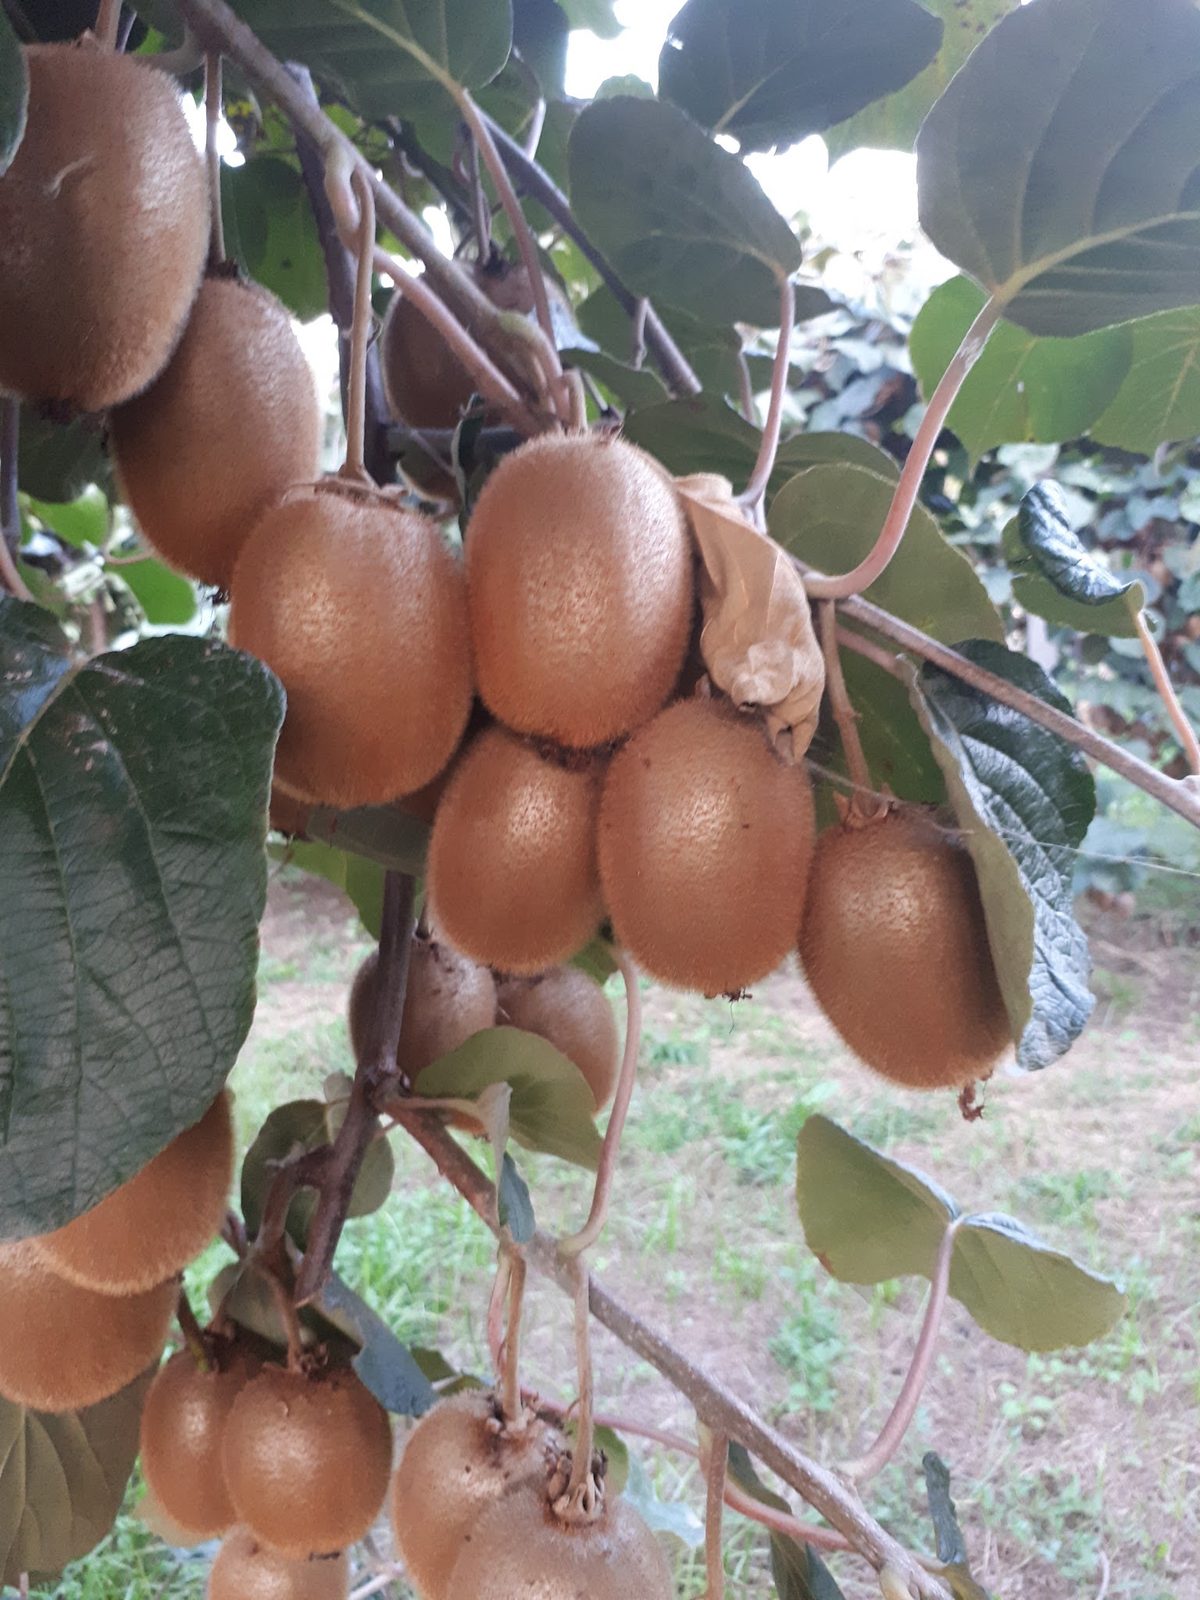
Kiwifruit (Actinidia deliciosa, cultivar ‘Hayward’) is a deciduous climbing vine and is functionally dioecious: the flowers form both whorls of reproductive organs, but on female vines the pollen is sterile and on male vines the ovary remains rudimentary. Morphologically the flowers look bisexual; functionally they are unisexual [1]. The fruit is a berry; in ‘Hayward’ the usual weight runs from 70 to 110 grams and rarely exceeds 140 [2].
The Greek crop now exceeds 15,000 hectares and 300,000 tonnes, which places the country consistently fourth in the world [3]. Despite the scale of the crop, bud physiology remains the least understood part of it, and it is precisely what determines fruit number.
Kiwifruit bears fruit only on current-season shoots arising from two-year-old wood. The flowers appear in the axils of the first leaves of the current-season shoot, and the wording has to be exact here: in the axils of the first leaves, not at the first buds of the one-year-old cane, because those first buds usually do not break at all. In ‘Hayward’ the zone carrying nearly all the flowers is nodes 6 to 12 [4]. The same pattern has been recorded in Actinidia arguta, where the most productive flowering zone on the shoot is likewise nodes 6 to 12, while canes produce fruitful shoots along their whole length with a maximum at nodes 6 to 26 [5].

2. The two-year cycle of the bud
In pome and stone fruit the flower bud differentiates in the same year it is formed. In olive and grapevine differentiation is completed at the end of the following winter [6] [7]. Kiwifruit follows the second model, and in an extreme form: the whole cycle from bud initiation to open flower is spread over two growing seasons, with a long winter in between [8] [9].
| Period | What happens inside the bud | What is visible outside |
|---|---|---|
| Spring, year A | The zero-order bud breaks. First-order axillary buds form in the leaf axils of the new shoot. | Rapid growth; flowers from last year's buds. |
| June to July, year A | The fate of each meristem is settled. Those above node 5 keep growing; the lower ones stop. | Nothing. The bud is just a swelling. |
| Summer to autumn, year A | Bud scales, leaf primordia and second-order structures are completed. No floral primordia at all. | Wood maturation, leaf fall. |
| Winter | Standstill. Sugars accumulate in the meristems. | Dormancy. This is when pruning is done. |
| Late winter, year B | Meristems at nodes 6 to 12 differentiate into inflorescences. Sepals, petals, stamens and pistil are formed. | Bud swell. |
| May, year B | Ovule initiation is completed. | Bloom, the second ten days of May in Pella. |
The table places the work on a Northern Hemisphere calendar. The New Zealand papers count in days after budbreak, so as to be independent of hemisphere.
3. What is inside a first-order axillary bud
The most detailed anatomical description comes from Walton and co-workers, who followed ‘Hayward’ buds through a full year [10]. The figures are specific and worth a grower knowing, because they explain everything else:
| Structure | Number per mature bud | What becomes of it |
|---|---|---|
| Bud scales and leaf primordia | 23 ± 2 | Protection, and the leaves of the future shoot |
| Second-order structures in total | about 16 | Split between the two categories below |
| Second-order axillary buds (nodes 1 to 4) | 4 | Usually never break |
| Simple dome-shaped meristems | 12 ± 4 | Node 5 usually aborts; nodes 6 to 12 give flowers; the more distal ones become next year's buds |
| Third-order meristems | 20 ± 6 | A reserve, in the axils of the second-order buds |


4. When flowering is decided: the moment of evocation
Evocation is the moment a meristem commits to becoming a flower rather than a shoot. It is invisible: nothing changes morphologically, what changes is the fate of the cells. For decades it was thought to occur in kiwifruit in late summer. Two independent approaches showed that it happens far earlier.
Snelgar and Manson defoliated shoots on successive dates and counted how many produced flowers the following spring. Their conclusion: in New Zealand evocation takes place during December and January, that is the first half of summer, which for Greece corresponds to June and July. Their estimate for the start was about 73 days after budbreak. And one finding of immediate practical value: each axillary bud is evoked at about the time the leaf below it stops expanding, while evocation proceeds progressively from the base of the shoot towards the tip [12].
The anatomical work arrived at the same point by another route. The meristems at node 5 and below stop increasing in size by day 68 after budbreak, while those at node 6 and above carry on. The parting of fates, some to become buds, some flowers, has already occurred by then or earlier. And it is no coincidence that the largest meristems sit exactly at nodes 6 to 12, where the flowers appear [10].
Morphological differentiation, by contrast, is a matter of spring. In a study on ‘Hayward’ and ‘Matua’, the reproductive meristem of ‘Hayward’ remained uninitiated until 12 days before budburst, five days behind the male ‘Matua’. Sepal primordia were evident before budburst, petal primordia at budburst, stamens at advanced budburst, and the pistil last. Pistillate flowers formed about a week after the staminate ones [13]. Under our conditions the process starts around 10 to 20 March and closes with bloom in the second ten days of May.
Bud biochemistry tells the same story. Through winter, sugars make up about 78% of the carbohydrates measured in the meristems, and sucrose more than 86% of those sugars, reaching 200 mg per gram of dry weight. Starch changes very little, while sucrose and hexoses rise rapidly from autumn to mid-winter [14].
5. The genetic confirmation
The strongest evidence came from molecular biology. The kiwifruit homologues of the Arabidopsis floral meristem identity genes LEAFY and APETALA1 were isolated and named ALF and AAP1. Their expression is bimodal: a first phase in late spring of the first growing season, exactly when the second-order meristems are initiated, and a second one roughly ten months later, when those meristems differentiate into flowers [15].
Where the expression sits is equally revealing. In the first spring ALF is expressed throughout the developing first-order bud, while AAP1 is localised in the second-order meristems. In the second spring both concentrate in the differentiating flowers. Which is to say, floral commitment is written into the bud in year one and executed in year two.
Sources: 15
6. Dormancy and its three faces
Dormancy is, in the classical definition, «the suspension of visible growth of any plant structure containing a meristem» [16]. That same paper introduced the distinction still in use, and it has direct practical consequences:
- Paradormancy. The inhibition comes from another part of the same plant, above all apical dominance. It is lifted by pruning or by changing the orientation of the cane.
- Endodormancy. The inhibition is internal to the bud itself. Nothing but chilling lifts it, however favourable the weather.
- Ecodormancy. The bud is ready but external conditions, cold, drought, prevent budbreak. It lifts of its own accord.
Dormancy is a survival mechanism: it makes sure the vine does not break bud during a warm week in January and get destroyed by the next frost [17] [18].
The transition from one state to another can be detected long before anything is visible. The respiration rate of buds, measured in autumn, correlates with the proportion of floral shoots and the number of flowers per bud the following spring, that is, it gives an indication of the crop seventeen weeks before budbreak. Buds from the coolest region consistently had the highest respiration rate. In spring a sharp rise follows, 3 to 6 weeks before budbreak [19].
7. Chilling hours or chilling units: a costly confusion
One number circulates whenever a new kiwifruit planting is discussed: «kiwifruit needs 750 to 800 chilling hours». The number is right but the unit is wrong, and the difference matters in the calculation.
There is a second caveat, rarely mentioned: the requirement of 750 to 800 units has never been tested experimentally on whole plants, and the suitability of the Richardson unit for kiwifruit itself is questioned by more than one group [20] [21]. What circulates as an absolute number is in reality an estimate.
What is consistently documented is this: temperatures up to 10 °C are effective in satisfying the chilling requirement, and ‘Hayward’ additionally needs a long frost-free growing season of the order of 220 days [20] [22]. Short days combined with high temperatures also deepen dormancy more than long days with alternating temperatures [22].
8. How many buds break, and why
In theory every overwintering bud, apart from the second-order ones, can break and carry flowers. In practice many lose that capacity or keep it in reduced form [23]. Budbreak along the cane is never uniform: it ranges from close to 0% near the base to 100% near the tip [24]. The distribution is structured, not random, and can be described with branching-sequence models [25].
Three factors stand out:
- Winter temperature. The proportion of buds producing floral shoots exceeds 50% after a cold winter and falls below 20% after a mild one [24] [21].
- Cane orientation. Vertical canes show a lower density of budbreak near the base, through apical dominance. Cane angle affects evocation, flower numbers and productivity [26] [27].
- Late frost. Even with the chilling requirement fully met, a frost shortly before budbreak destroys the buds. In Greece the March 2025 frost cut national production by roughly 20% [3].
No correlation has been found between budbreak and phyllotaxis [26] [1].
Sources: 1 3 21 23 24 25 26 27
9. Breaking dormancy: what the research shows and what is permitted
The international literature on dormancy-breaking agents, and on hydrogen cyanamide in particular, is extensive and broadly favourable as regards performance. Application increases and synchronises budbreak, increases the number of canes bearing flowers, and improves floral differentiation [28] [29]. At the anatomical level, application 35 days before expected natural budbreak at 1, 2 and 3% advanced differentiation so far that, when the controls were only forming sepals in 57.6% of buds, the treated vines had almost completed stamen formation [30]. At the molecular level the compound triggers a very rapid transcriptional activation, mostly of stress-response genes and secondarily of genes associated with the reactivation of growth [31]. Alternative approaches such as exogenous cytokinins have also been investigated [32].
That, however, does not mean the material is off the market. Every year the Ministry grants DORMEX 52 SL an emergency authorisation of 120 days under Article 53 of the same regulation, for limited and controlled use on kiwifruit in named regional units, among them Pella, Imathia, Pieria, Thessaloniki, Larisa, Fthiotida, Arta, Preveza, Aitoloakarnania, Kavala and Xanthi [39].
Even where it is permitted, the tool has a cost. Application advances budbreak and so exposes the planting to late frosts [28] [29]. In a climate where a March frost cost one fifth of national production, advancing budbreak is not a neutral choice.
Sources: 28 29 30 31 32 33 34 39
10. Nitrogen, vigour and flowering
The relationship between nitrogen and flowering in kiwifruit is one of the points on which the literature does not agree, and that deserves saying plainly rather than picking the convenient side.
| Study | Finding | The authors' interpretation |
|---|---|---|
| Smith and Miller, 1992 | More buds broke on vines heavily fertilised the previous year | Attributed to the osmotic effect of the fertiliser rather than to nutrition as such [35] |
| Vizzotto et al., 1999 | Fewer fruit produced on canes with excess nitrogen, and greater sensitivity to winter frost | Excess nitrogen degrades both quality and hardiness [36] |
| Buwalda et al., 1990 | Development and effects of nitrogen deficiency in a field planting | Deficiency is as limiting as excess [37] |
| Testoni et al., 1990 | Effect of mineral nutrition on yield and quality | Points in the same direction as the previous study [38] |
The fertiliser rates in these studies apply to the conditions under which they were run and do not transfer unchanged. What transfers is the direction: excess nitrogen does not buy flowers, and it raises the risk from frost.
The practical consequence is not “less nitrogen”. It is that the rate should follow from a calculation rather than from habit: expected yield, soil organic matter, soil and leaf analysis, the general vigour of the planting, and the nitrate content of the irrigation water, which in many boreholes in Pella is not negligible and is rarely taken into account.
11. What all this means at pruning
The five things that change in practice
- Select canes of spring origin. A bud is evoked when the leaf below it stops expanding [12]. Canes that started in spring have completed evocation along almost their whole length. Canes that grew after midsummer did not, and will give fewer flowers whatever is done over winter.
- Do not count the first five nodes. The first four are second-order buds that do not break, and the meristem of the fifth usually aborts [10] [11]. A cane with “twenty buds” actually has fifteen usable ones.
- Leave enough length. Since the flowering zone is nodes 6 to 12, every cane must comfortably reach beyond the twelfth node [4]. Pruning too short cuts off precisely the productive zone.
- Lay canes horizontal. A vertical cane breaks very few buds near its base, through apical dominance [27]. The angle is not a matter of how the row looks; it is a matter of how many buds will wake up.
- Protect the canopy in June and July. That is the window of evocation [12]. Loss of leaf area then costs the crop of the following year.
On fertile sites in our area, 22 to 25 canes per vine are usually retained, each with 12 to 25 axillary buds, and in some cases up to 30 canes. The number is not a rule; it is a function of planting distances, vigour and expected budbreak, and the right way to set it is to measure last season's budbreak in the same block rather than copy a figure from the neighbouring one.
12. Sources
The numbers in the text refer to the list below.
- [1] Ferguson, A.R. (1990). Stem, branches, leaves and roots of the kiwifruit vine. In: Kiwifruit: Science and Management (Warrington I.J. & Weston G.C., eds), pp. 58 to 70. New Zealand Society for Horticultural Science, Wellington. Source for cane morphology, the functionally dioecious habit, and the absence of any correlation between budbreak and phyllotaxis.
- [2] Hopping, M.E. (1988). Leaf area, final fruit weight and productivity in kiwifruit. Scientia Horticulturae. Source for the typical ‘Hayward’ fruit weight, 104 and 110 grams in the two years of the trial.
- [3] Greece, fresh kiwifruit production and trade (FAO data). Source for the 317,080 tonnes of 2023, fourth place worldwide, roughly 15,000 hectares, and the loss of about 20% from the March 2025 frost.
- [4] Walton, E.F. & Fowke, P.J. (1993). Effect of hydrogen cyanamide on kiwifruit shoot flower number and position. Journal of Horticultural Science 68:529-534. Source for the flowering zone at nodes 6 to 12 and for the number of meristems that differentiate into inflorescences.
- [5] Tiyayon, C. & Strik, B. (2003). Flowering and fruiting morphology of hardy kiwifruit, Actinidia arguta. Acta Horticulturae 610:171-176. Source for confirmation of the 6 to 12 zone in a second species, for the productive zone at nodes 6 to 26, and for 47% budbreak with 83% floral shoots.
- [6] Tufts, W.P. & Morrow, E.B. (1925). Fruit-bud differentiation in deciduous fruits. Hilgardia 1:1-14. Source for same-year differentiation in pome and stone fruit.
- [7] Hartmann, H.T. (1951). Time of floral differentiation of the olive in California. Botanical Gazette 112:323-327; Pratt, C. (1971). Reproductive anatomy of cultivated grapes. American Journal of Enology and Viticulture 22:92-109. Source for the olive and grapevine model, where differentiation is completed in the spring of anthesis.
- [8] Brundell, D.J. (1975a). Flower development of the Chinese gooseberry (Actinidia chinensis Planch.). I. Development of the flower shoot. New Zealand Journal of Botany 13:473-483. First description of the two-year cycle and of the basal second-order buds.
- [9] Brundell, D.J. (1975b). Flower development of the Chinese gooseberry. II. Development of the flowering bud. New Zealand Journal of Botany 13:485-496. Source for the differentiation of floral organs after winter dormancy.
- [10] Walton, E.F., Fowke, P.J., Weis, K. & McLeay, P.L. (1997). Shoot axillary bud morphogenesis in kiwifruit (Actinidia deliciosa). Annals of Botany 80:13-21. Source for all the anatomical figures: 23±2 bud scales and leaf primordia, about 16 second-order structures, 4 second-order buds, 12±4 dome-shaped meristems, 20±6 third-order meristems, completion by day 125, abortion of node 5, and the arrest of basal meristem growth by day 68.
- [11] Snowball, A.M. (1997). Seasonal cycle of shoot development in selected Actinidia species. New Zealand Journal of Crop and Horticultural Science 25:221-231. Source for the distinction between first- and second-order axillary buds and for the failure of the latter to break.
- [12] Snelgar, W.P. & Manson, P.J. (1992). Determination of the time of flower evocation in kiwifruit vines. New Zealand Journal of Crop and Horticultural Science 20:439-447. Source for evocation in December to January in New Zealand, for a start about 73 days after budbreak, for the progression from base to tip, and for the link with the end of expansion of the subtending leaf.
- [13] Gökbayrak, Z., Söylemezoğlu, G., Engin, H. & Dardeniz, A. (2010). Examination of flower bud differentiation and development in kiwifruit. Journal of Biology & Life Sciences 1(1):1-4. Source for ‘Hayward’ remaining uninitiated until 12 days before budburst, for the five-day difference from ‘Matua’, and for the order of sepal, petal, stamen and pistil formation.
- [14] Richardson, A.C., Walton, E.F., Meekings, J.S. & Boldingh, H.L. (2010). Carbohydrate changes in kiwifruit buds during the onset and release from dormancy. Scientia Horticulturae 124:463-468. Source for sugars at 78% of measured carbohydrates, sucrose at 86% of the sugars, 200 mg per gram of dry weight, and the stability of starch through winter.
- [15] Walton, E.F., Podivinsky, E. & Wu, R.-M. (2001). Bimodal patterns of floral gene expression over the two seasons that kiwifruit flowers develop. Physiologia Plantarum 111:396-404. Source for the ALF and AAP1 genes, for bimodal expression ten months apart, and for the localisation of expression in each phase.
- [16] Lang, G.A., Early, J.D., Martin, G.C. & Darnell, R.L. (1987). Endo-, para- and ecodormancy: physiological terminology and classification for dormancy research. HortScience 22:371-377. Source for the definition of dormancy and the distinction between the three types.
- [17] Horvath, D.P., Anderson, J.V., Chao, W.S. & Foley, M.E. (2003). Knowing when to grow: signals regulating bud dormancy. Trends in Plant Science 8(11):534-540. Source for the agronomic importance of understanding dormancy mechanisms.
- [18] Rohde, A. & Bhalerao, R.P. (2007). Plant dormancy in the perennial context. Trends in Plant Science 12(5):217-223. Source for dormancy as a survival mechanism of perennials against seasonal conditions.
- [19] McPherson, H.G., Snelgar, W.P., Manson, P.J. & Snowball, A.M. (1997). Bud respiration and dormancy of kiwifruit (Actinidia deliciosa). Annals of Botany 80:411-418. Source for the correlation of autumn bud respiration with flowering, for the 17-week forecasting horizon, and for the spring rise 3 to 6 weeks before budbreak.
- [20] Sibley, J.L., Dozier, W.A., Pitts, J.A., Caylor, A.W., Himelrick, D.G. & Ebel, R.C. (2005). Kiwifruit cultivars differ in response to winter chilling. Small Fruits Review 4(4):19-29. Source for the distinction between Richardson units and hours, for Caldwell's 900 and 1,150 hours, for the 220 frost-free days, for the effectiveness of temperatures up to 10 °C, and for the caveat that the 750 to 800 units have never been tested on whole plants.
- [21] McPherson, H.G., Stanley, C.J. & Warrington, I.J. (1995). The response of bud break and flowering to cool winter temperatures in kiwifruit (Actinidia deliciosa). Journal of Horticultural Science 70:737-747. Source for the response of budbreak and flowering to cool winter temperatures and for doubts over the Richardson unit in kiwifruit.
- [22] Lionakis, S.M. & Schwabe, W.W. (1984). Bud dormancy in the kiwi fruit, Actinidia chinensis Planch. Annals of Botany 54:467-484. Source for the effectiveness of temperatures up to 10 °C and for the effect of photoperiod and temperature on the depth of dormancy.
- [23] Grant, J.A. & Ryugo, K. (1982). Influence of developing shoots on flowering potential of dormant buds of Actinidia chinensis. HortScience 17:977-978. Source for the loss of flowering capacity in part of the overwintering buds.
- [24] McPherson, H.G., Hall, A.J. & Stanley, C.J. (1994). Seasonal and regional variation in budbreak and flowering of kiwifruit vines in New Zealand. New Zealand Journal of Crop and Horticultural Science 22:263-276. Source for the budbreak gradient from 0% at the base to 100% at the tip and for the difference in floral shoots between cold and mild winters.
- [25] Guédon, Y., Barthélémy, D., Caraglio, Y. & Costes, E. (2001). Pattern analysis in branching and axillary flowering sequences. Journal of Theoretical Biology 212:481-520. Source for the structured, non-random distribution of budbreak and flowering along the shoot.
- [26] Costa, G., Vizzotto, G. & Testolin, R. (1991). Kiwifruit: variations in vegetative gradient and cropping performance as related to cane orientation. Advances in Horticultural Science 5:15-18. Source for the effect of cane orientation on final budbreak and for the absence of correlation with phyllotaxis.
- [27] Snelgar, W.P. & Manson, P.J. (1990). Influence of cane angle on flower evocation, flower numbers, and productivity of kiwifruit vines. New Zealand Journal of Crop and Horticultural Science 18(4):225-232. Source for reduced budbreak at the base of vertical canes and for the effect of angle on flower numbers.
- [28] Costa, G., Vizzotto, G. & Lain, O. (1995 and 1997). Fruiting performance of kiwifruit cv. Hayward affected by use of hydrogen cyanamide. Acta Horticulturae 444:473-478. Source for the increase in budbreak and flowering after application, and for the risk of advancing budbreak.
- [29] Linsley-Noakes, G.C. (1989). Improving flowering of kiwifruit in climatically marginal areas using hydrogen cyanamide. Scientia Horticulturae 38:247-259. Source for use in sites marginal for chilling and for the resulting early budbreak.
- [30] Engin, H., Gökbayrak, Z. & Dardeniz, A. (2010). Effects of hydrogen cyanamide on the floral morphogenesis of kiwifruit buds. Chilean Journal of Agricultural Research 70(3):503-509. Source for application 35 days before expected budbreak at 1, 2 and 3%, and for 57.6% of controls with sepal primordia while treated buds had reached stamen formation.
- [31] Walton, E.F. et al. (2009). A rapid transcriptional activation is induced by the dormancy-breaking chemical hydrogen cyanamide in kiwifruit (Actinidia deliciosa) buds. Journal of Experimental Botany 60(13):3835-3848. Source for the transcriptional response, with most induced genes related to stress and a subset to the reactivation of growth.
- [32] Fabbroni, C. (2009). Kiwifruit bud release from dormancy: effect of exogenous cytokinins. PhD thesis, Università di Bologna. Source for the investigation of alternatives to hydrogen cyanamide.
- [33] Cyanamide, Pesticide Properties Database (PPDB), AERU, University of Hertfordshire. Source for the “not approved” status of cyanamide under Regulation (EC) 1107/2009 and for the expiry of its inclusion.
- [34] Database of authorised plant protection products and biocides, Greek Ministry of Rural Development and Food (September 2026 edition; in Greek, valid in Greece only). Source for the 142 authorised uses in kiwifruit and for the absence of any dormancy-breaking product among them.
- [35] Smith, G.S. & Miller, S.A. (1992). Osmotic effects on performance and fruit quality of kiwifruit vines. Acta Horticulturae 297:331-336. Source for increased budbreak after heavy fertilisation and for attributing it to an osmotic rather than a nutritional cause.
- [36] Vizzotto, G., Lain, O. & Costa, G. (1999). Relationship between nitrogen and fruit quality in kiwifruit. Acta Horticulturae 498:165-172. Source for reduced fruit numbers on canes with excess nitrogen and for the increased sensitivity of the buds to winter frost.
- [37] Buwalda, J.G., Wilson, G.J. & Smith, G.S. (1990). The development and effects of nitrogen deficiency in field-grown kiwifruit (Actinidia deliciosa) vines. Plant and Soil 129:173-182. Source for the effects of nitrogen deficiency in a real planting.
- [38] Testoni, A., Granelli, G. & Pagano, A. (1990). Mineral nutrition influence on the yield and the quality of kiwi fruit. Acta Horticulturae 282:203-208. Source for the relationship between mineral nutrition, yield and quality.
- [39] DORMEX 52 SL: grant of a 120-day authorisation for limited and controlled use on kiwifruit. Greek Ministry of Rural Development and Food, ref. 9442/276074, 20 December 2022 (in Greek). Source for the Article 53 emergency authorisation and for the list of regional units it covers. The authorisation is re-issued each year by a new decision.
Photographs: Pastopoulos Agronomics archive, Neos Mylotopos, Pella, November 2021.
Related articles
Training kiwifruit: T-bar and pergola
The architecture of the kiwifruit vine and why both training systems follow from it. T-bar and pergola with their dimensions, advantages, costs and a comparison in numbers. Training from the day of planting: planting high, a first season for the root with tipping at one metre, cutting back low the following spring and taking the trunk up in the second season, leaders, winter and summer pruning, males and the support structure. Three diagrams, a table of mistakes, and the gaps that remain for Greece. A field observation from Giannitsa on planting distances.
Copper nanoparticles for kiwifruit bacterial canker
A Chinese study compared three copper nanomaterials with a conventional bactericide. On the plate they needed concentrations at least sixty four times lower. On the plant the control efficacies fell into the same range…
Chilling hours: the three models and when each one tells the truth
Chilling Hours, Utah Chill Units or Dynamic Chill Portions, what each measures, which suits which climate and season, why a chill portion does not convert into hours, and how the divergence between the three is read. The calculation itself lives in a separate tool.